该研究考察适应(adaptation,即重复抑制,repetition suppression)对下颞叶(IT)神经元物体编码准确性的具体影响。作者利用单细胞与多单元两组电生理数据进行信号检测论判别力(d′)与群体解码分析,发现重复呈现相同刺激会降低神经判别力,而在测试刺激与前置适配刺激不同的交叉适应条件下,判别力反而可获得特异性提升,表明短期适应具有优先表征新异刺激的自适应编码特性。
研究背景
IT 神经元在刺激重复后常出现明显反应下降,人类 fMRI 适应范式也利用类似现象推断脑区的刺激表征。但“反应变小”本身并不能说明编码变好还是变差:若重复使调谐更锐利,判别力可能提高;若只是压缩反应差,物体之间反而更难区分。早期视觉区的部分研究曾发现适应提高刺激判别力,符合高效编码的设想,而 IT 的重复抑制更强,却不能据此直接推断同一功能后果。fMRI 中关于调谐锐化、平均化或反应缩小的争论,也需要神经层面的判别力指标来澄清。
关键还在于区分重复与交叉适应。若适应具有刺激特异性,刚出现过的刺激受到更强抑制,那么后续两个测试刺激的反应分布可能靠近,也可能拉开,方向取决于先前刺激是偏好还是非偏好。只比较适应前后平均放电,会把这两种相反结果混在一起。判别力 d′ 能同时考虑均值差和试次变异,群体分类器则可检验下游读出是否真正获益。由此,研究问题从“重复抑制有多大”转为“适应后物体身份还能被多准确地分辨”。
本文重分析两组猕猴 IT 数据:一组用参数化渐变形状测单细胞 d′,另一组用同步多通道 MUA 做群体解码。不同 adapter–test 组合分别检验完全重复、交替呈现和只有一方重复的情况,并用时间窗分析检查重复是否仅使加工更快。结果显示,重复通常降低判别力,而某些交叉适应可增强,主要由均值反应差改变而非方差变化驱动。这支持适应偏向新异信息的解释,但结论限于短间隔、无插入刺激的被动观看;长延迟、重复启动和长期熟悉化可能遵循不同规律。
研究思路
研究重新分析了两组实验数据,采用信号检测论的敏感度指标 d′ 和群体线性解码器评估神经判别力,使适配刺激(adapter)与测试刺激(test)间的形状差异沿参数化维度渐变,用以系统分离单纯刺激重复与交叉适应的效应。其逻辑在于:若适应具有刺激特异性(即对重复呈现的刺激抑制幅度大于对新异刺激的抑制),则当先前适应于弱反应刺激时,后续强反应与弱反应刺激间的响应差异将被拉大,d′ 应当升高;反之,若先前适应于强反应刺激,两者的响应差异被压缩,d′ 应当下降。
实验一基于单细胞记录评估参数化渐变形状的调谐,考察单个神经元的判别力改变;实验二采用 16 通道层状探针记录同步多单元活动(MUA)并进行群体解码,评估跨通道群体读出是否与单细胞水平一致。此外,通过滑动时间窗分析检验重复刺激是否表现为反应潜伏期前移的易化加工。
方法
实验一(单细胞):2 只恒河猴,共记录 80 个具有显著视觉选择性的 IT 神经元(每只猴各 40 个)。刺激包含 4 组经 morph 渐变生成的三维带阴影形状(每组 6 个渐变级,高度 5.4°–7.2°,面积与平均灰度配平),于注视中央凹呈现。测定形状选择性后开展适应测试:6 个渐变等级互为适配与测试刺激,构成 36 种序列组合,每张图片呈现 300 ms,刺激间间隔(ISI)为 300 ms;注视窗口为 ≤2°,维持注视获得果汁奖励;每个适应试次后插入两个打乱噪点图像以消退适应残留,每种条件平均包含 8.11 个有效试次。
实验二(MUA 群体):2 只恒河猴(其中 1 只参与了实验一),使用 16 通道层状探针(触点间距 100 μm)记录 STS 下岸皮层活动,共完成 32 次穿透,记录到 468 个反应位点。每次穿透从 52 张彩色物体图片中挑选两张诱发响应差异明显的图片作为测试刺激;每张图片呈现 500 ms,ISI 为 500 ms,试次分为重复序列(AA/BB)与交替序列(AB/BA);重点分析刺激呈现后 60–310 ms 的早期时段。
判别力指标计算为 d′ = |M(P)−M(L)|/√((σ²(P)+σ²(L))/2),其中 P 代表神经元的偏好刺激,L 代表沿渐变轴偏离 1–3 个等级的较弱刺激;在 MUA 分析中,P 与 L 分别定义为该记录位点在初始呈现时诱发最大与最小反应的两个刺激。群体解码采用基于相关的线性分类器(每次穿透最多包含 16 个有效通道,经 1000 次交叉验证,机会水平 50%),分别测试在当前条件下独立训练以及仅利用适配刺激基线响应进行固化读出两种分类方案。
主要结果
- 重复降低单神经元判别力:以 d′ 评估,在完全重复试次中(Test(PP, LL)),测试刺激的判别力显著低于其作为适配刺激呈现时及交替试次中(Test(PL, LP));前置适应刺激为偏好形状时(Test(PP, PL))同样显著拉低 d′;而前置适应刺激为非偏好形状时(Test(LL, LP))呈现轻微上升趋势,但事后检验未达显著(p=0.22)。在单细胞水平,测试刺激相对适配刺激的放电率中位数下降了 22%。渐变形状距离主效应显著(F(2,158)=39.746),适应条件主效应显著(F(4,316)=17.061)(图 2A)。
- d′ 改变主要由均值反应差异驱动,而非方差变异:在重复试次中,重复呈现的偏好刺激被抑制的绝对幅度更大(单细胞放电率:Test(PP) 为 34.72 spikes/s,Test(LP) 为 39.87 spikes/s),而反应方差与均值的比值(Fano 因子)变动轻微(适配刺激时为 0.90,测试刺激时为 1.2–1.3),判别力下降可由各刺激均值差的相对压缩充分解释(表 1、表 2)。
- 交叉适应可反向提升特定形状对的判别力:在偏好形状位于渐变轴极值端的神经元亚群中(n=26),当前置适配刺激为反应最弱的极端形状(等级 5)时,测试偏好形状对的 d′ 显著高于适配刺激基线水平(p=0.0201);而当前置适配刺激为偏好形状时,判别力显著降低(p=0.0014)。然而,该交叉增强效应并未在非偏好形状对的测试中重现(p=0.8093),表明判别力提升依赖于适配刺激与测试刺激在调谐曲线上的相对位置(图 3、表 3)。
- MUA 群体呈现更显著的适应分化:条件主效应高度显著(F(4,1868)=209.56);Test(PP, LL) 的 d′ 显著低于基线与交替条件,而 Test(LL, LP) 的 d′ 则显著超出基线与交替测试条件(均 p<10⁻⁶)。放电抑制普遍存在(在 90% 的“刺激×记录点”组合中均可检测到),且主要集中在刺激诱发反应的前半段(图 2B、图 4A)。
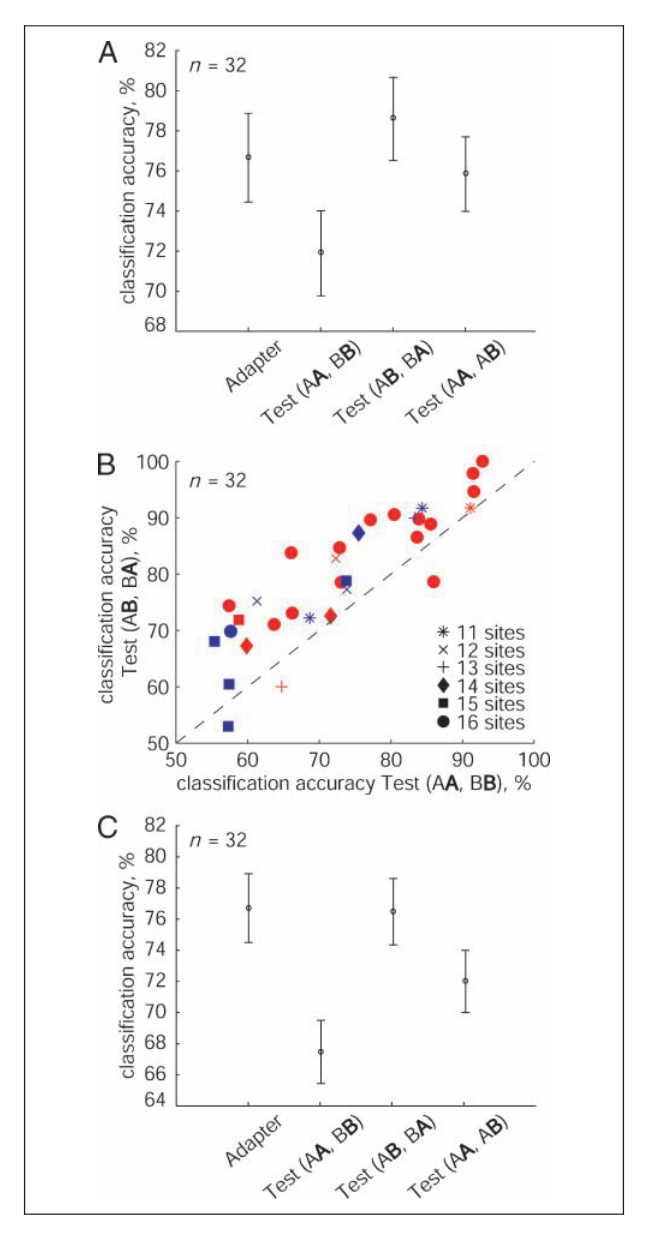
- 群体解码准确率的调制:利用局部小群体(中位数 15.5 个位点)进行分类,重复测试刺激的解码准确率最低(72%),交替测试刺激最高(79%),Test(AA, AB) 条件居中(76%),适配刺激基线为 77%;32 次穿透中仅 3 次未表现出重复引起的准确率下降。在固化读出模式下(仅使用适配刺激数据训练分类器),重复测试刺激的准确率依然显著低于基线(67% 对 77%,p<10⁻⁶)。时间进程分析显示,短至 12.5 ms 的滑动窗口已能提供高于机会水平的解码能力,解码准确率随窗口拓宽至 50 ms 达到渐近线;刺激重复主要压低了信息量的峰值幅度,并未改变信息到达峰值的时间点,这与反应时易化假说不符(图 4、图 6)。
图注解读
图 1 · 刺激与适应范式
原文图注:Figure 1. Stimuli and adaptation paradigm. (A) Illustration of one set of shapes employed in the single cell study (Experiment 1). The letters serve to identify each of the shapes. (B) Schematic of adaptation test with two of the images employed in the simultaneous MUA recordings study (Experiment 2). Top and bottom illustrate a repetition and alternation trial, respectively. In both experiments, the animals were required to fixate a small fixation target (shown here not to scale) presented at the center of a monitor for 500 msec before stimulus onset (FIX). The adapter (S1) and test (S2) stimuli were shown for 300 and 500 msec in Experiments 1 and 2, respectively, and separated by an ISI of the same duration as the stimulus. Monkeys were required to fixate during the entire trial, including the poststimuli (POST) interval, lasting 300 and 475 msec in Experiments 1 and 2, respectively. Successful fixation throughout a trial was rewarded by a drop of apple juice.
读法:A 为实验一所用的参数化 morph 渐变形状示例,B 为实验二的时序结构。两个实验均采用两段式刺激呈现(S1 适配,S2 测试),刺激时长与中间 ISI 在实验一中均为 300 ms,在实验二中均为 500 ms,猴需在全程保持注视。该示意图界定了重复与交替试次的时间间隔与刺激呈现方式,是判读后文各类条件代号的基础。
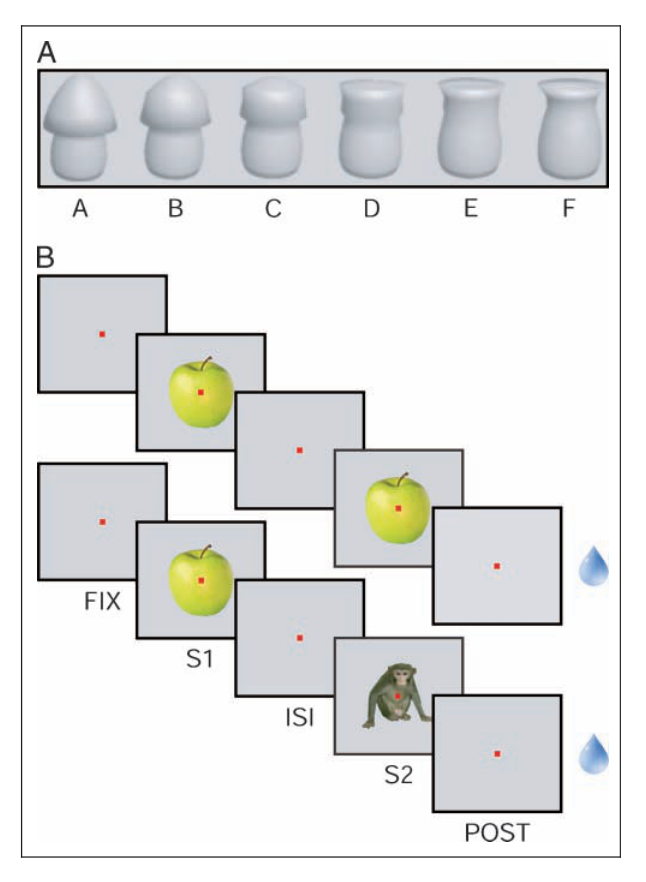
图 2 · 五种适应条件下的 d′
原文图注:Figure 2. Mean discriminability index d0 for adapter and test stimuli across different adaptation conditions. (A) Mean d0 of single neurons (n = 80) measured at three different distances (D) between the preferred (P) and less preferred (L) shapes for five different conditions: shapes presented as adapter, shapes presented as test in repetition trials (Test(PP, LL)), shapes presented as test in alternation trials (Test(PL, LP)), and shapes presented as test of which one was following an identical adapter and the other shape was following the different adapter (Test(PP, PL) and Test(LL, LP)). (B) Mean d0 of MUA activity (n = 468 responsive sites) for the same five conditions as in A. Each MUA site was stimulated by two stimuli P and L that were defined as the stimuli eliciting the largest and smallest response, respectively, when presented as adapter. In both A and B, bars indicate standard errors of the mean and bold letters correspond to the stimulus pairs for which d0 was computed.
读法:横轴排列五种条件(基线 Adapter、Test(PP, LL)、Test(PL, LP)、Test(PP, PL) 与 Test(LL, LP)),纵轴表示平均判别力 d′。核心特征显示:Test(PP, LL) 在单细胞(A)与多单元群体(B)中均显著低于基线与交替条件,反映单纯重复抑制会压缩判别力;而在 Test(LL, LP) 条件下,群体层面呈现出显著高于基线的判别力提升,单细胞层面表现出同向趋势。本图支持主要结果第 1、4 条。
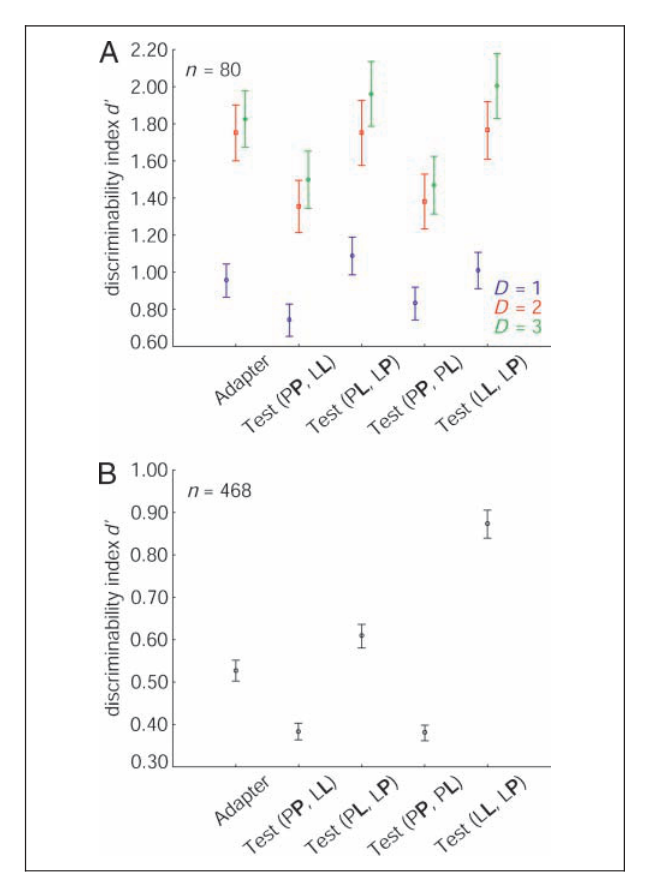
图 3 · 适配器沿形状维取值对 d′ 的调制
原文图注:Figure 3. Mean discriminability index d0 of single IT neurons plotted as a function of the adapter value of the parameterized shape. Adapter value: 1 = preferred shape; 5 = less preferred shape differing by 4 values from the adapter. (A) d0 computed for the preferred shape (value = 1) and the shape with value 3 (i.e., distance = 2) presented as tests. (B) d0 computed for the less preferred shape with value 5 and the shape with value 3 (i.e., distance = 2) presented as tests. The d0 value for the same shapes presented as adapters is indicated by the stippled horizontal line. Only the neurons (n = 26) for which the preferred shape was either an extreme (A and F in Figure 1A) or differed by one value from the extreme (B and E in Figure 1A) were considered for this analysis. Bars indicate standard errors of the mean. Insets: schematic monotonic tuning curves with stimuli used to compute d0 indicated by filled, gray circles and connected by a thick black line.
读法:横轴表示适配刺激在渐变形状轴上的等级(1 为该细胞的偏好形状,5 为最弱反应形状),虚线表示该形状对在适配基线时的 d′ 水平。A 针对偏好形状对进行测试:当适配刺激为偏好形状时,d′ 显著低于基线;当适配刺激为非偏好形状时,d′ 显著高于基线。B 针对非偏好形状对测试,曲线两端均未偏离基线。插图示意了单调调谐曲线上刺激差被拉大或压缩的几何机制,支持主要结果第 3 条。
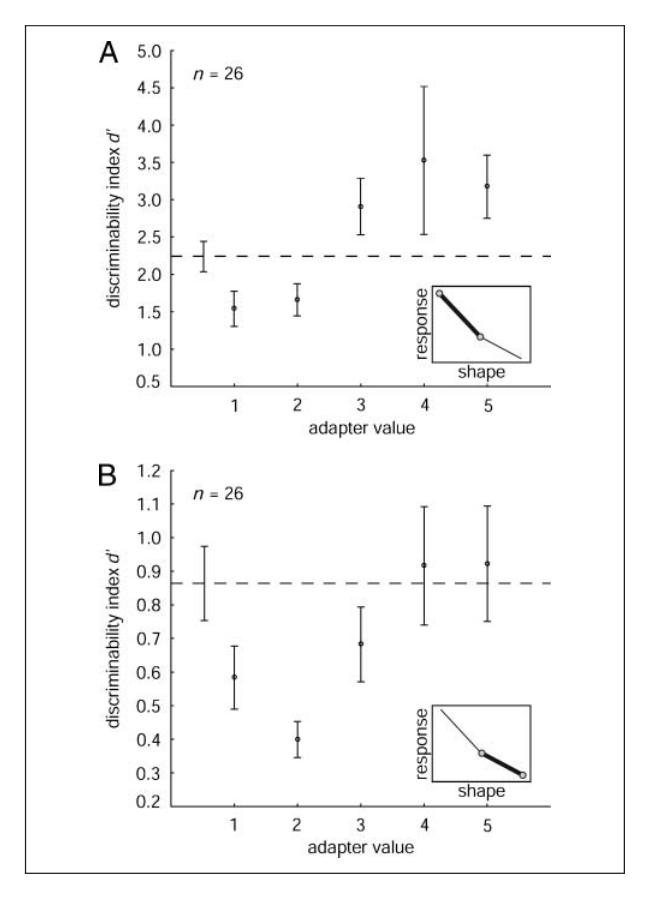
图 4 · MUA 与解码精度的时间进程
原文图注:Figure 4. Time course of MUA and classification accuracy. (A) Population PSTH of the mean spiking activity, averaged across all responsive recording sites of both animals, in repetition (Rep trials) and alternation (Alt trials) trials. Responses are aligned on the onset of the adapter stimulus. Stippled vertical lines indicate stimulus on- and offsets. Firing rates were computed with a sliding window of 50 msec with a step of 10 msec. (B) Mean classification accuracy computed with different sliding window durations (see legend) for repetition trials (AA and BB trials). Mean accuracies are plotted at the center of the corresponding window (e.g., accuracy for the 0–50 msec window plotted at 25 msec); 0 msec corresponds to the onset of the adapter stimulus. Chance level is 50%. (C) Mean classification accuracy for four adaptation conditions (see legend), obtained with a sliding window of 50 msec and aligned on stimulus onset. Mean classification accuracy obtained when shuffling the stimulus labels across trials of a condition (Shuffled) were computed using the same sliding windows and did not differ from the chance level (50%). Training and testing was done for each condition and window separately using the correlation-based classifier. Vertical stippled lines indicate stimulus on- and offset. Bands indicate standard errors of the mean.
读法:A 为群体发放率的刺激后时间直方图(PSTH),显示重复抑制主要集中在反应起始后的前半段。B 为采用 12.5–100 ms 不同滑动窗计算的解码准确率时间轨迹,显示短窗口下准确率依然稳健,且重复测试刺激在各时相的峰值均低于基线,但峰值出现时间并未前移。C 展示了四种条件下 50 ms 窗长的分类轨迹,重复测试刺激全程处于最低水平。本图支持主要结果第 5 条。
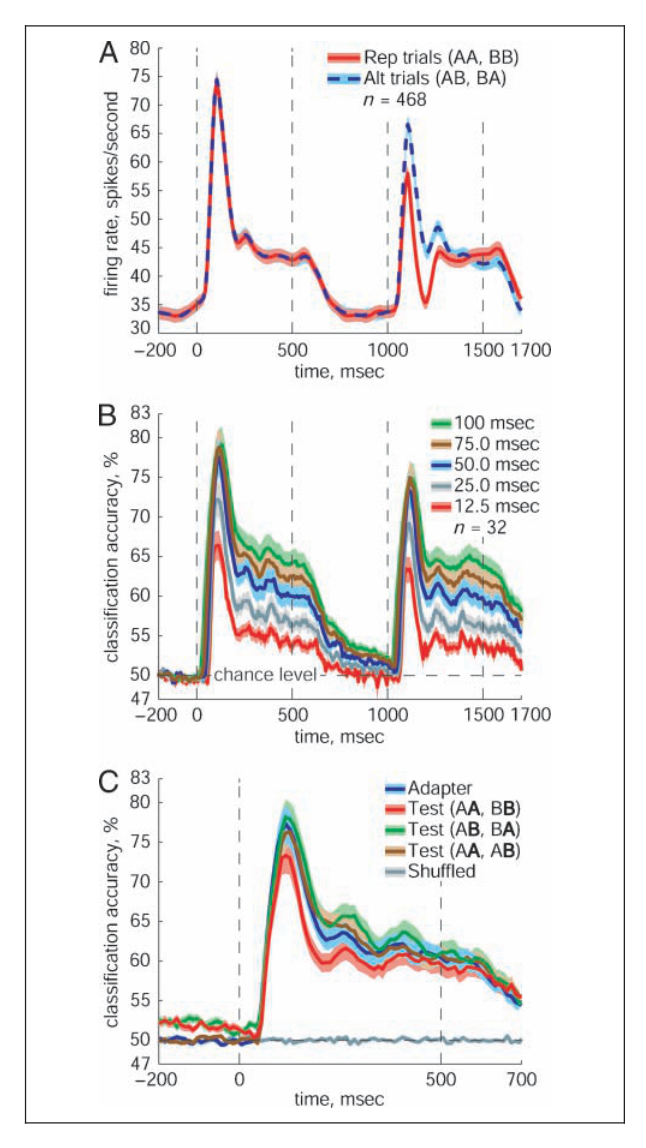
图 5 · d′ 变化的机制示意
原文图注:Figure 5. Illustration of effects of adaptation on neuronal discriminability. The two distributions in each row represent the responses to the P (solid line) and L (stippled line) stimuli. Top row: response distributions for stimuli presented as adapter; middle row: response distributions for stimuli when adapting to P; bottom row: response distributions for stimuli when adapting to L. Adaptation to P produces a larger reduction of the response to the repeated stimulus P than to L, resulting in a decreased discriminability. When adapting to L, the response to the repeated stimulus L is more suppressed compared with the response to P, which enhances discriminability between them. The Fano factor was equated for all response distributions. Note that the distributions do not represent real, recorded data but serve to explain graphically the differential effects of adaptation to P and L stimuli.
读法:本图为概念示意模型。上行表示初始基线时偏好刺激 P(实线)与非偏好刺激 L(虚线)的响应分布。中行显示适应于 P 时的效应:P 分布受到的抑制更大,两分布间距缩小,导致判别力降低。下行显示适应于 L 时的效应:L 分布受到更强抑制,两分布间距拉大,导致判别力提升。模型固定了各分布的 Fano 因子,说明平均响应差的改变足以解释 d′ 的双向变化。
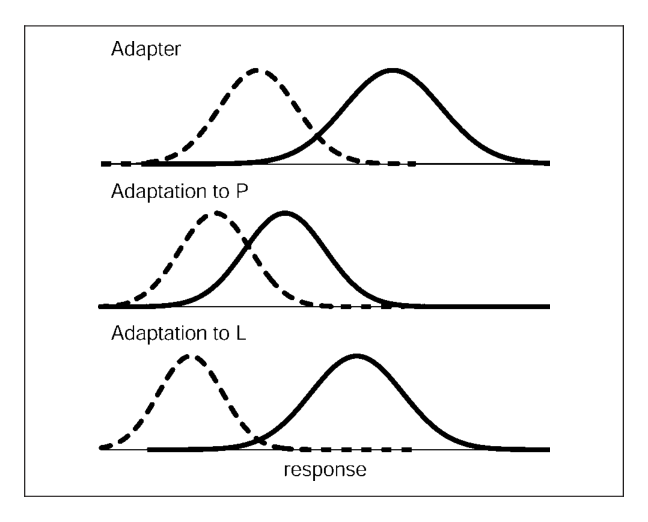
图 6 · 群体分类精度与读出方式
原文图注:Figure 6. Classification accuracy (n = 32 penetrations) of MUA. (A) Mean classification plotted for four adaptation conditions: adapter stimulus, test stimulus in repetition trials (Test(AA, BB)), test stimulus in alternation trials (Test(AB, BA)), and the average of two conditions Test(AA, AB) and Test(BB, BA) (here indicated by Test(AA, AB)). Classification accuracies were obtained when training and testing classifiers on the data of each condition separately. Bars indicate standard errors of the mean, and bold letters correspond to the stimuli for which classification was performed. (B) Classification accuracy for the test stimuli in alternation trials plotted against the classification accuracy for the same stimuli in repetition trials. Each point corresponds to a single penetration. Different symbols and colors label penetrations according to the number of responsive sites of a penetration and animal, respectively. The diagonal is indicated by a stippled line. (C) Mean classification plotted for four adaptation conditions when the classifiers were trained only with response vectors for the adapter stimuli and then tested for each condition. Abbreviations are the same as in A.
读法:A 为各条件独立训练测试时的群体解码表现,重复测试刺激准确率显著偏低。B 为散点图,横轴为重复测试刺激准确率,纵轴为交替测试刺激准确率;绝大多数点分布于对角线上方,表明交替刺激的读出准确率系统性优于重复刺激。C 采用固定分类器(仅利用适配刺激基线训练),重复测试刺激的读出缺陷依然存在,证实该现象不依赖于解码器权重在各条件下的自适应调整。本图支持主要结果第 5 条。
讨论
本研究的电生理分析表明:在缺乏间隔任务的短时间隔重复呈现下,IT 神经元对重复刺激的判别力发生降低。这一效应在单细胞与多单元两组独立数据中均得到验证,且在不同尺度的分析窗口下保持稳定,表明短时重复并不普遍增强局部特征的表征精度;而在交替序列中,当前置刺激与测试刺激相异时,神经判别力可以出现选择性提升。d′ 的变化主要由刺激特异性抑制引起的平均放电率差距改变所主导,反应方差的变异未构成主导贡献。在功能层面,在眼动扫描与连续注视过程中,该机制有助于降低对刚感知过的已知物体的编码冗余,同时相对提高对新出现物体的神经敏感度,符合感觉系统在连续输入下优化动态范围与代谢成本的组织特征。
研究同时界定了结论的边界条件:实验设置基于数百毫秒尺度的短时呈现且中间缺乏干扰任务;而在长延迟间隔或存在插入刺激的情境下(如部分 fMRI 研究所涉及的长时程设计),重复呈现可能表现出不同的表征演化。在与其他区域的对比中,本数据未检测到支持“重复提升低频同步以补偿放电下降”计算模型的普遍证据;与部分初级或中级视觉皮层(如 V4 或 MT)在特定适应参数下观察到的微弱判别力增益相比,IT 皮层表现出的明显判别力抑制更多体现了高阶形状表征在短时适应下的特有动态。最后,本实验的短时适应效应不应直接等同于行为层面的重复启动或长期的知觉学习过程。
一句话总结
本实验从判别力指标切入,明确了下颞叶神经元适应现象的功能特性:刺激特异性抑制并非无差异地削弱或提升感知表征,而是依据测试刺激与前置适配刺激在调谐维度上的相对关系对判别力产生双向调节;研究结合单细胞与多通道电生理记录,证实短时重复主要导致相同物体的区分度降低,而对新异刺激的相对区分能力得以保持或选择性提升。